Monday, September 24, 2018

3033. On the Coming Economic Downturn

By Ruchir Sharma, The New York Times, September 19, 2018
The central bankers Ponzi game
After the fall of Lehman Brothers 10 years ago, there was a public debate about how the leading American banks had grown “too big to fail.” But that debate overlooked the larger story, about how the global markets where stocks, bonds and other financial assets are traded had grown worrisomely large.

By the eve of the 2008 crisis, global financial markets dwarfed the global economy. Those markets had tripled over the previous three decades to 347 percent of the world’s gross economic output, driven up by easy money pouring out of central banks. That is one major reason that the ripple effects of Lehman’s fall were large enough to cause the worst downturn since the Great Depression.

Today the markets are even larger, having grown to 360 percent of global G.D.P., a record high. And financial authorities — trained to focus more on how markets respond to economic risk than on the risks that markets pose to the economy — have been inadvertently fueling this new threat.
Over the past decade, the world’s largest central banks — in the United States, Europe, China and Japan — have expanded their balance sheets from less than $5 trillion to more than $17 trillion in an effort to promote the recovery. Much of that newly printed money has found its way into the financial markets, where it often follows the path of least regulation.

Central bankers and other regulators have largely succeeded in containing the practice that caused disaster in 2008: risky mortgage lending by big banks. But with so much easy money sloshing around in global markets, new threats were bound to emerge — in places the regulators aren’t watching as closely.

Within the $290 trillion global financial markets, there are hundreds of new risks, pools of potentially troubled debt. Among the most troubling: corporate borrowers and so-called non-bank lenders all over the world.

As bank lending dried up, more and more companies began raising money by selling bonds, and many of those bonds are now held by these non-bank lenders — mainly money managers such as bond funds, pension funds or insurance companies.

Among corporations listed on the S.&P. 500 index, debt has tripled since 2010 to one and a half times annual earnings — near the historic peaks reached during the recessions of the early 1990s and 2000s. And in some parts of the bond markets, debt loads are much higher.

One of the big corporate risks is developing largely beyond regulatory oversight. Some United States companies that were publicly traded in 2008 have since gone private, often precisely in order to avoid intensified scrutiny from regulators. Many of those companies were purchased by private equity firms, in deals that leave the companies saddled with huge debts. Right now the typical American company owned by a private equity firm has debt six times higher than its annual earnings — or twice the level that a public ratings agency would consider high-risk or “junk.”

At a time when central banks are holding interest rates at record lows, the return from holding plain vanilla corporate bonds is negligible, so investors are more willing to buy junk, for the higher yields. And this hunt for higher returns has been playing out worldwide as asset managers chase higher returns anywhere they can be found, whether in United States private equity or in the bond markets of Europe and emerging economies like Argentina and Turkey.

The biggest risks outside the United States are in China, which has printed by far the most money and issued by far the most debt of any country since 2008, and where regulators have had less success reining in borrowers and lenders. Easy money has fueled bubbles in everything from stocks and bonds to property in China, and it’s hard to see how or when these bubbles might set off a major crisis in an opaque market where most of the borrowers and lenders are backed by the state. But if and when Beijing reaches the point where it can’t print any more money, the bottom could fall out of the economy.

More broadly, the trigger to watch is the United States Federal Reserve, since many other central banks in the world tend to follow the Fed’s lead in setting interest rates. Over the last 50 years, every time the Fed has reined in easy money by raising interest rates, a downturn in the markets or the economy has followed eventually. It may take a while, but trouble almost inevitably does come.

Many doomsayers worried that the Fed tightening that began in 2004 would help prompt a recession — and it eventually did, in 2008. Though rates are still historically low in the United States, the Federal Reserve began to raise them more than two years ago and is expected to continue tightening them into next year.

The Fed’s tightening is already rattling emerging markets. When the American markets start feeling it, the results are likely be very different from 2008 —  corporate meltdowns rather than mortgage defaults, and bond and pension funds affected before big investment banks.

If a downturn follows, it is more likely to be a normal recession than another 100-year storm, like 2008. Most economists put the probability of such a recession hitting before the end of 2020 at less than 20 percent.

But economists are more often wrong than right. Professional forecasters have missed every recession since such records were first kept in 1968, and one of the many reasons for this is “recency bias”: using economic forecasting models that tend to give too much weight to recent events. They see, for example, that big banks are in much better shape than in 2008, and households are less encumbered by mortgage debt, and so play down the likelihood of another recession. But they are, in effect, preparing to fight the last war.

To have any chance of anticipating and preventing the next downturn, regulators must look for the threats that have emerged since 2008. They need to recognize that the markets now play an outsized role in the economy, and their attempts to micromanage this vast sea of money have only pushed the risks away from big American banks and toward new lenders outside the banking system, particularly in the United States and China.

Markets have grown so large in part because every time they stumbled, central bankers rescued them with easy money. When markets rose sharply — as they have in recent years — the authorities stood by, saying they are not in the business of popping bubbles. Now, the markets are so large it is hard to see how policymakers can lower the risks they pose without precipitating a sharp decline that is bound to damage the economy. It’s a familiar problem: Like the big banks in 2008, the global markets have grown “too big to fail.”

Ruchir Sharma is the chief global strategist at Morgan Stanley Investment Management.  

3032. Terrestrial Primary Production: Fuel for Life

By Knowledge Project, The Nature Education, No Date

Terrestrial ecosystems rely almost exclusively on the sun's energy to support the growth and metabolism of their resident organisms. Plants are quite literally biomass factories powered by sunlight, supplying organisms higher up the food chain with energy and the structural building blocks of life. Land plants, or autotrophs, are terrestrial primary producers: organisms that manufacture, through photosynthesis, new organic molecules such as carbohydrates and lipids from raw inorganic materials (CO2, water, mineral nutrients). These newly minted organic compounds lock up the sun's energy in chemical bonds, providing an energy currency accessible to heterotrophs, organisms that consume rather than produce organic molecules. In this way, primary producers are an essential vehicle for energy transfer from the sun to consumers, securing energy that can be passed from one consumer to another. The energetic and carbon-rich products of primary production supply consumers, including humans, with fuel to drive their metabolism while providing essential carbon-containing compounds that form the bricks and mortar of living cells.
Ecosystem ecologists have long been interested in two related metrics of terrestrial primary production. Gross primary production (GPP) is the total amount of carbon dioxide "fixed" by land plants per unit time through the photosynthetic reduction of CO2 into organic compounds. A substantial fraction of GPP supports plant autotrophic respiration (Ra), with the remainder allocated to the net primary production (NPP) of plant structural biomass in stems, leaves, and fruit, labile carbohydrates such as sugars and starch, and, to a much lesser extent, volatile organic compounds used in plant defense and signaling. Terrestrial GPP, therefore, relates to NPP as follows:
NPP = GPP - Ra
Net primary production (NPP) and standing biomass allocation for a 90-year-old Michigan forest estimated from inventory-based methods in which biomass growth is quantified over time (Gough <i>et al.</i> 2008)
Figure 1: Net primary production (NPP) and standing biomass allocation for a 90-year-old Michigan forest estimated from inventory-based methods in which biomass growth is quantified over time (Gough et al.2008)
© 2011 Nature Education All rights reserved. View Terms of Use
Both GPP and NPP are expressed as rates, usually in terms of their carbon currency (e.g., g C m-2 hr-1, tonnes C ha-1 yr-1). Because volatile organic compounds represent only a small fraction of NPP, the rate of total plant growth (or yield) in a terrestrial ecosystem is virtually synonymous with NPP, since biomass production is already discounted for respiratory expenditures that support plant growth and maintenance. The ratio of NPP to GPP, or carbon use efficiency, is the fraction of carbon absorbed by an ecosystem that is allocated to plant biomass production. Interestingly, carbon use efficiency is often remarkably similar across ecosystems located in different biomes, suggesting that ecosystems organize in a way that maximizes carbon allocation to growth.
Where do plants invest organic compounds designated for net primary production? Consider, as an example, a mature forest. The stems, leaves, flowers, and fruit are all visible displays of aboveground NPP (i.e., growth) that accrued over time — but what about belowground (root) NPP? Most of the NPP readily observed aboveground is matched in magnitude belowground by the less visible, but equally important, production of roots. For example, root growth comprised almost half of total ecosystem NPP in a ninety-year-old Michigan forest, indicating that belowground investments in biomass by plants are substantial (Figure 1). The total standing biomass of an ecosystem is a function of cumulative NPP over time minus biomass losses from senescence (i.e., death). In the same forest, stems (including trunks and branches) are the largest fraction of standing biomass, but roots comprise a quarter of the total biomass present in the ecosystem.

Measuring Gross and Net Primary Production

Meteorological towers like this one located in a temperate forest are distributed across ecosystems in all continents except Antarctica, providing assessments of carbon uptake by forest, grassland, desert, and crop ecosystems.
Figure 2: Meteorological towers like this one located in a temperate forest are distributed across ecosystems in all continents except Antarctica, providing assessments of carbon uptake by forest, grassland, desert, and crop ecosystems.
© 2011 Nature Education All rights reserved. View Terms of Use
Scientists use several complementary tools for quantifying terrestrial gross and net primary production at ecosystem to global scales. On-the-ground inventory based methods are commonly used in cropland, grassland, and forested ecosystems to measure NPP. This approach requires estimates of biomass production through periodic measurements of root, stem, leaf, and fruit growth. The growth over time of all plant tissues within a terrestrial ecosystem is equal to NPP. In this approach, aboveground (ears, stalks, leaves) and belowground (roots) corn biomass yield over a single growing season is equal to annual NPP of this crop ecosystem.
Recent technological advances also allow for on-the-ground estimates of terrestrial primary production using meteorological towers that measure the uptake or emissions of CO2 by ecosystems (Figure 2). Meteorological towers measure net ecosystem CO2 exchange (NEE), which is equal to GPP minus ecosystem respiration or the quantity of CO2 respired by both autotrophs (plants) and heterotrophs (primarily microbes). GPP and NPP are calculated indirectly by adding ecosystem and heterotrophic respiration, respectively, to NEE. Meteorological approaches are employed worldwide in forest, agricultural, grassland, and desert ecosystems to track terrestrial primary production. For example, the international research network FLUXNET (Baldocchi et al.2001) supports observations of terrestrial primary production on six of seven continents.
At the global scale, satellite data combined with mathematical modeling is essential to providing worldwide estimates of terrestrial primary production. Several approaches have been used, but most notable are products derived from NASA's Moderate-resolution Imaging Spectroradiometer (MODIS), a satellite-mounted instrument that collects surface spectral, or color, data useful for tracking changes in the productivity of terrestrial and marine ecosystems. An example MODIS product is a "greenness" index of the Earth's surface used to estimate terrestrial primary production. Surface greenness and other remotely sensed data collected from space provide coarser assessments of NPP and GPP than inventory and meteorological tower based methods but have the advantage of providing estimates of terrestrial primary production for large areas where ground-based methods are not feasible.

Terrestrial Primary Production Over Time and Across the Earth's Surface

Patterns of terrestrial NPP at different timescales in a temperate forest: Daily net primary production (NPP) changes during the growing season in response to climate variables including solar radiation and precipitation, while the duration of NPP during the growing season (i.e., spring green-up to autumn leaf fall) is largely a function of photoperiod. Annual NPP changes from one year to the next in response to longer-term trends in climate, including shifts in total solar radiation caused by differences in cloud cover from year to year. Decadal patterns of NPP track changes in ecological succession (Gough <i>et al.</i> 2007, 2008).
Figure 3: Patterns of terrestrial NPP at different timescales in a temperate forest: Daily net primary production (NPP) changes during the growing season in response to climate variables including solar radiation and precipitation, while the duration of NPP during the growing season (i.e., spring green-up to autumn leaf fall) is largely a function of photoperiod. Annual NPP changes from one year to the next in response to longer-term trends in climate, including shifts in total solar radiation caused by differences in cloud cover from year to year. Decadal patterns of NPP track changes in ecological succession (Gough et al. 2007, 2008).
© 2011 Nature Education All rights reserved. View Terms of Use
Terrestrial primary production fluctuates over time and is closely coupled with physical (i.e., abiotic) and ecological (i.e., biotic) changes that play out over different timescales. On scales of seconds to hours, primary production during the growing season responds to environmental drivers of photosynthesis, generally increasing with photosynthetic photon flux density (PPFD) or the spectrum of solar radiation available to power photosynthesis. At the seasonal scale, terrestrial primary production of boreal and temperate ecosystems is tied to changes in temperature and photoperiod, or day length, (Figure 3) while in tropical regions seasonal precipitation patterns often dictate cycles of high and low primary production. Year-to-year, or interannual, changes in terrestrial primary production are often related to long-term climate variation including prolonged drought and, in some cases, variation from one year to the next in average annual temperature and solar radiation.
Over decades, a period that is meaningful to ecological succession, terrestrial primary production changes in response to shifts in plant competition and disturbance. Consider an abandoned field that undergoes a successional reversion back to forest. Plant communities will assemble during early succession, with fast-growing plants emerging first and because of low initial plant density there will be little competition for resources. As a result, total plant growth in the ecosystem, or NPP, will proceed at an increasingly higher rate for several years. NPP generally levels off or declines once plants start crowding one another and begin competing more intensively for limiting light, nutrient, and water resources (Figure 3). Terrestrial primary production also may change over time in response to natural disturbances such as insect outbreaks, wind, fire, and pathogens that diminish photosynthesis by reducing leaf biomass and causing plant death. Long-term increases in atmospheric CO2 and nitrogen deposition associated primarily with fossil fuel burning generally increase plant growth over long periods of time.
Terrestrial primary production varies considerably across the surface of the Earth and among different ecosystem types. Terrestrial primary production, both NPP and GPP, vary from north to south (or latitudinally) due to gradients in plant community composition, growing season length, precipitation, temperature, and solar radiation. However, east to west (longitudinal) differences in terrestrial primary production also exist. These spatial differences are illustrated in a map of global NPP derived from NASA's MODIS satellite (Figure 4). For example, there is a precipitous decline in NPP from east to west in middle North America that is largely a function of declining precipitation. NPP generally declines from tropical regions to the poles because of temperature and light limitations. Tropical forests tend to be much more productive than other terrestrial ecosystems, with temperate forests, tropical savannah, croplands, and boreal forests all exhibiting middle levels of primary production (Table 1). Desert and Tundra Biomes, limited by precipitation and temperature respectively, contain the least productive ecosystems. In addition to climatic regulation of terrestrial primary production, disturbance, management, and land-use change (including urbanization) play critical roles in determining spatial differences in terrestrial primary production.
The global distribution of land and ocean net primary production (NPP) estimated from spectral data gathered by NASA's MODIS satellite
Figure 4: The global distribution of land and ocean net primary production (NPP) estimated from spectral data gathered by NASA's MODIS satellite
Public Domain NASA Earth Observatory.
Tropical ecosystems, because of their high productivity and extensive footprint on the Earth's surface, comprise nearly half of global NPP and GPP (Table 1). Temperate ecosystems and croplands are also a substantial fraction of global terrestrial primary production, accounting for roughly a quarter of global NPP and GPP. Global estimates of terrestrial NPP range from 48.0 to 69.0 Pg (= Petagrams or 1015 g) C yr-1, with global terrestrial GPP estimated at 121.7 Pg C yr-1 or approximately double global NPP on land.
Biome Global GPP1 
(Pg C yr
 -1)
Global NPP2 (PG C yr-1)Ecosystem NPP3 (g C ha-1 yr 
Tropical forest40.816.0–23.1871–1098
Temperate forest9.94.6–9.1465–741
Boreal forest 8.32.6–4.6173–238
Tropical savannah and grasslands 31.314.9–19.2343–393
Temperate grasslands and shrublands8.53.4–7.0129–342
Deserts6.40.5–3.528–151
Tundra1.60.5–1.080–130
Croplands14.84.1–8.0288–468
TOTAL121.748.0–69.0 2377–3561
Table 1: Global and ecosystem-scale estimates of mean terrestrial gross and net primary production for the Earth's major biomes from remotely sensed satellite data and modeling students. 1 Petagram (Pg) = 1015 grams (g).
1. Beer et al. 2000; 2. Melillo et al. 1993; Potter et al. 1993; Prince & Goward 1995; Field et al. 1998; Beer et al. 2010 3. Melillo et al. 1993; Potter et al. 1993; Prince & Goward 1995 
Haberl et al. (2007) estimated that nearly a quarter of global NPP is used by humans annually in the production of crops for food and fiber, timber for wood products and paper, and in support of livestock grazing. Humans exert an additional influence on global NPP through fires. Many ecologists are concerned that the rising global demand for biofuels, together with continued human population growth, will increase this already large human appropriation of global NPP to the detriment of ecological food webs and biodiversity.

Terrestrial Primary Production and Global Change

Considerable research in ecosystem ecology centers on understanding how climate change is affecting the primary production of terrestrial ecosystems and, conversely, how ecosystems may moderate changes in global climate by absorbing anthropogenic CO2emissions. Terrestrial primary production is an important ecosystem service, locking up carbon in biomass that might otherwise exist in the atmosphere as CO2, a potent greenhouse gas. Recent evidence suggests, however, that terrestrial NPP may be declining in response to global warming and accompanying drought, with Zhoa & Running (2010) estimating a 0.55 Pg, or about 1%, reduction in global terrestrial NPP from 2000 to 2009. Continued declines in global NPP would not only reduce carbon sequestration by terrestrial ecosystems but also compromise food security and disrupt the foundation of food webs.

Summary

Ecosystem ecologists have long been interested in quantifying and understanding what controls terrestrial primary production. While gross primary production (GPP) is the total influx of carbon into an ecosystem through the photosynthetic fixation of CO2, net primary production (NPP) is this gross carbon influx discounted for plant respiratory costs of growth and maintenance. Net primary production forms the base of ecological food chains and is heavily manipulated by humans in the production of food, fiber, wood, and increasingly biofuels. Climate, disturbance, and ecological succession exert influences on terrestrial NPP and GPP, suggesting that mounting anthropogenic influences on global climate and land-use will have substantial effects on the future primary production of terrestrial ecosystems.

References and Recommended Reading


Baldocchi, D. et al. FLUXNET: A new tool to study the temporal and spatial variability of ecosystem-scale carbon dioxide, water vapor, and energy flux densities. Bulletin of the American Meteorological Society 82, 2415–2434 (2001).
Beer, C. et al. Terrestrial gross carbon dioxide uptake: Global distribution and covariation with climate. Science 329, 834–838 (2010).
Field, C. B. et al. Primary production of the biosphere: Integrating terrestrial and oceanic components. Science 281, 237–240 (1998).
Gough, C. M. et al. The legacy of harvest and fire on ecosystem carbon storage in a north temperate forest. Global Change Biology 13, 1935–1949 (2007).
Gough, C. M. et al. Controls on annual forest carbon storage: Lessons from the past and predictions for the future. Bioscience 58, 609–622 (2008).
Haberl, H. et al. Quantifying and mapping the human appropriation of net primary production in earth's terrestrial ecosystems. Proceedings of the National Academy of Sciences USA 104, 12942–12945 (2007).
Melillo, J. M. et al. Global climate-change and terrestrial net primary production. Nature 363, 234–240 (1993).
Potter, C. S. et al. Terrestrial ecosystem production - a process model-based on global satellite and surface data. Global Biogeochemical Cycles 7, 811–841 (1993).
Prince, S. D. & Goward, S. N. Global primary production: A remote sensing approach. Journal of Biogeography 22, 815–835. 1995.
Roy, J. et al. Terrestrial Global Productivity. San Diego, CA: Academic Press (2001).
Zhao, M. S. & Running, S. W. Drought-induced reduction in global terrestrial net primary production from 2000 through 2009. Science329, 940–943 (2010).

Sunday, September 23, 2018

3031. Global Human Appropriation of Net Primary Production Doubled in the 20th Century

By Fridolin Krausmann, Karl-Heinz Erb, Simone Gingrich, Helmut Haberl, Alberte Bondeau, Veronika Gaube, Christian Lauk, Christoph Plutzar, and Timothy D. Searchinger, 
Proceeding of the National Academy of Sciences of the United States of America, June 18, 2013


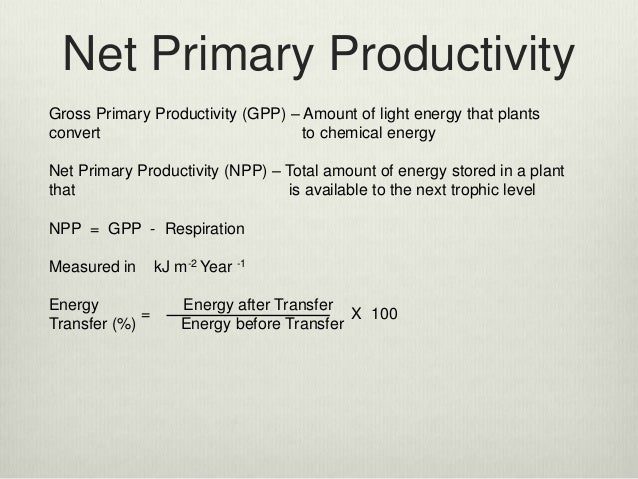
Ultimately, all species live off energy that arrives on Earth via sunshine.  Through photosynthesis green plants (primary producers) convert solar energy into sugars. They consume about half of it for their own livelihood. What remains is called Net Primary Productivity (NPP).  The NPP is the basis for all animal life. Herbivores eat plants to gain energy for their livelihood (primary consumers). Finally, some carnivores live off herbivores (secondary consumers).  Some omnivores eat secondary consumers (tertiary consumers).  The final link in the food chain is the decomposers that live off the organic matter of plants, herbivores and carnivores.  In each step in the food chain about 90% of the energy is lost. 

Abstract


Global increases in population, consumption, and gross domestic product raise concerns about the sustainability of the current and future use of natural resources. The human appropriation of net primary production (HANPP) provides a useful measure of human intervention into the biosphere. The productive capacity of land is appropriated by harvesting or burning biomass and by converting natural ecosystems to managed lands with lower productivity. This work analyzes trends in HANPP from 1910 to 2005 and finds that although human population has grown fourfold and economic output 17-fold, global HANPP has only doubled. Despite this increase in efficiency, HANPP has still risen from 6.9 Gt of carbon per y in 1910 to 14.8 GtC/y in 2005, i.e., from 13% to 25% of the net primary production of potential vegetation. Biomass harvested per capita and year has slightly declined despite growth in consumption because of a decline in reliance on bioenergy and higher conversion efficiencies of primary biomass to products. The rise in efficiency is overwhelmingly due to increased crop yields, albeit frequently associated with substantial ecological costs, such as fossil energy inputs, soil degradation, and biodiversity loss. If humans can maintain the past trend lines in efficiency gains, we estimate that HANPP might only grow to 27–29% by 2050, but providing large amounts of bioenergy could increase global HANPP to 44%. This result calls for caution in refocusing the energy economy on land-based resources and for strategies that foster the continuation of increases in land-use efficiency without excessively increasing ecological costs of intensification.
Although planet earth is finite, the growth of world population and economic activity result in an increasing demand for natural resources and ecosystem services. Concerns about these trends have motivated prominent scholars to define a new geological era, the “anthropocene” (1, 2). Changes in land use are particularly pervasive (3, 4) because human activities now affect approximately three-quarters of all vegetated lands (5). In the next four decades, population is expected to grow by 40% (6), the world economy could grow by a factor of 3 over its present value (7), and agricultural production is expected to grow by 60–100% (8, 9). Moreover, influential energy strategies advocate expanding bioenergy severalfold from its present value of ∼50 exajoule (EJ)/y (10, 11). At the same time, there are concerns that humanity is already outside its safe operating space in terms of nitrogen use, climate change, and biodiversity loss and near other critical limits such as land use (12) or biomass production of green plants (13). The ability of humanity to respect planetary boundaries (12) will depend on its ability to decouple growth from its demand for resources (14).
The capacity of land to produce biomass is one critical limiting resource (13). Although humans can influence that capacity through inputs and management, net primary production (NPP) is limited by land area, water, solar radiation, and soils. Biomass provides humans with food, fiber, and fuel, but it is also an indispensable resource for all other animals and microorganisms. Its annual production replenishes the carbon in soils and vegetation that is consumed by those animals and microorganisms and returned to the atmosphere (15) and, in some areas, generates the terrestrial carbon sink that helps to hold down climate change (16).
The human appropriation of the earth’s land capacity to produce biomass provides a useful measure of the human alteration of the biosphere. In previous work (17), we have defined this appropriation by the term “HANPP” for human appropriation of net primary production, which is the total carbon produced annually by plant growth. Total HANPP, measured in units of carbon, is the sum of two subcategories: HANPPluc and HANPPharv. HANPPharv is the quantity of carbon in biomass harvested or otherwise consumed by people, including crops, timber, harvested crop residues, forest slash, forages consumed by livestock, and biomass lost to human-induced fires. HANPPluc is the change in NPP, also measured as annual carbon flow, as a result of human-induced land use change, such as the conversion of forest to cropland or infrastructure. The calculation of HANPPlucrequires the estimation of the NPP that would be generated by the potential natural vegetation if vegetation were left unaltered, which we term NPPpot. We estimate NPPpot by using the global vegetation model Lund Potsdam Jena (LPJ) (SI Appendix), and use statistical data and thematic maps to estimate other inputs to HANPP (SI Appendix). From NPPpot, we can also calculate HANPP as a percentage of the potential productivity.
Because the carbon content of biomass is closely associated with its energy content, HANPP provides a set of indicators for measuring human effects on flows of trophic energy in natural ecosystems and managed lands (15, 17). HANPP can be used to calculate the intensity and the efficiency with which each hectare of land is used. Previous papers estimated HANPP and its major components for the 1980s (15, 18) and the year 2000 (17, 19, 20).
In this work, we present a global time series of HANPP over the last century, disaggregating by world regions and land use type. The goal is to provide insights into how changes in population and the economy have altered HANPP (21) that can be used to project future scenarios and to appreciate the implications of different policies that affect land use. Based on these data, we address several questions: (i) How much, and at what pace, did the human impact on the biosphere, measured by HANPP, change over the last century? (ii) How have global megatrends like growth of population and GDP influenced HANPP? (iii) To what extent have people improved their efficiency in using the land’s potential productivity to meet their needs and, thereby, decoupled HANPP from population and economic growth? (iv) How have regional patterns of HANPP changed, and what explains those differences? (v) How might HANPP evolve in the coming decades if current trends were to continue, and how would a strong increase in bioenergy demand alter the picture?

Results

During the last century, total human appropriation of plant growth has almost doubled (Fig. 1A). Global HANPP measured in GtC/y grew by 116% and by 2005 reached 14.8 GtC/y. As a percentage of the potential plant growth of native vegetation (NPPpot), HANPP grew from 13% in 1910 to 25% in 2005.
Although HANPP grew, it grew at a far slower rate than population and the economy. During the same period, population grew by 274% and gross domestic product (GDP) (in constant 1990 dollars) grew by 1,655% (22). HANPP per capita has therefore declined from a world average of roughly 3.9 tC/cap per y to 2.3 tons of carbon per capita and y. The major per capita decline in HANPP occurred only after 1950, when HANPP was still 3.7 tC/cap per y. HANPP per dollar of GDP (1990 dollars) declined even more throughout this century from 2.5 kilogram of carbon/$ to 0.3 kgC/$ (Fig. 1D).
Despite uncertainties in the data and assumptions, these results are robust. Fig. 1B shows upper and lower estimates of the HANPP trajectory in the 20th century. These estimates take into account uncertainties of data on biomass harvest and of assumptions on HANPPluc due to soil erosion and deforestation (SI Appendix), which results in a growth rate of HANPP from 99 to 129%. Because data regarding population and GDP are much less uncertain, the ranges in efficiencies are therefore also comparable.
Although total HANPP per capita declined, the level of biomass consumed by each person has remained nearly constant. As shown in Fig. 1C, global biomass harvest (HANPPharv) and consumption of biomass products have risen in almost perfect correlation with global population growth. That is a rather remarkable result because per capita consumption of crops and animal products for food has increased greatly along with use of timber for products other than energy. Indeed, food production per capita has risen since 1961 by an average of 20% in all world regions except the former Soviet Union (SI Appendix, Fig. S1B). However, decline in bioenergy has offset these increases (SI Appendix, Fig. S1A). Overall, wood harvest per capita has declined because of the replacement of fuel wood by fossil fuels. At the same time, the replacement of draft animals by tractors freed up agricultural land for other crops, and in some regions, allowed some lands to revert to forests. For example, before 1950 in Austria, 15–20% of all agricultural land and biomass use was required to feed draft animals that were later replaced by fossil-fuel powered machinery (23). This reduction in draft power has probably been lower in regions where animal draft power played a smaller role and in parts of the developing world where animal power is still important today (24). Although efficiency gains contributed to the decline of HANPP per dollar, the lion’s share of that reduction was due to a decreasing reliance on food and timber harvest for total economic production.

Land Use Efficiency.

In the first half of the 20th century, the extraction of 1 ton of carbon in biomass for human use resulted in roughly 2.1 tons of HANPP in the global average. This ratio means that each ton of plants harvested required the manipulation of land that reduced total biomass production by more than an additional ton. However, by 2005, that ratio had declined to 1.6. This improvement in land use efficiency resulted from technological changes that progressed differently across the globe (see Regional HANPP Trends below).
In general, the improvement has occurred overwhelmingly because of the rise in crop yields. In the vast majority of the world’s lands, converting forest and grassland to cropland reduces NPP. Although irrigation and heavy use of fertilizer have increased NPP in specific regions such as the Nile delta or The Netherlands even above NPPpot, most croplands have lower NPP due to the shorter growing period of crops and to the inability of one or a few crops to use the total solar radiation and other productive resources as fully as a mix of native species (17). However, by increasing yields over the last 50 y, farmers brought cropland closer to replicating the productivity of native vegetation, which meant that HANPPluc decreased (Fig. 2). Per unit area, HANPPluc on cropland declined from 235 to 117 gC/m2 per y (Fig. 2B). That led to a decrease in the absolute quantity of HANPPluc on cropland from a peak in 1950 at 2.3 GtC/y to 1.6 GtC/y by 2005. In fact, HANPPluc was slightly lower in 2005 even than 1910 despite almost a doubling of cropped area from 7 million km2 to 13 million km2. As a consequence, HANPPluc on cropland as a percentage of NPPpot declined from 49 to 21%. That also meant that the share of harvest in total HANPP grew from 55% in 1910 to 70% in 2005.
Fig. 2.
HANPP on global croplands. Development of harvested NPP (HANPPharv) and productivity losses due to land change (HANPPluc) compared with potential NPP (NPPpot) and NPP remaining in ecosystems after harvest (NPPeco). Absolute values (GtC/y) in A; per unit of cropped area (gC/m2 per y) in B.
Unlike rising crop yields, increasing harvest from forest land and the expansion of land occupied by infrastructure, buildings, and associated land have contributed to increasing HANPP (Fig. 1A). However, they have played a relatively small role because agriculture dominates HANPP globally, representing 84–86% of total appropriation of plant growth over the entire period, with 42–46% on cropland and 29–33% on grazing land.
By contrast with cropland, we here assume that the land use efficiency of pasture and forest did not increase. Because of the lack of reliable data and contradicting evidence from case studies on how grazing and forestry impact NPP, we assumed HANPPluc to be zero for woodland and for nondegraded natural grasslands for the observed time period. We did, however, consider HANPPluc resulting from conversion of forests to grasslands or urban land and from soil degradation (SI Appendix).
Although we did not assume any decline in HANPPluc on grasslands over time as a result of rising grassland productivity, the output of meat and milk has grown greatly relative to the harvest of grass. In 1961, when reliable production data first exist, 29 tons of grazed biomass (dry matter) were used for the production of 1 ton of animal products; by 2005, this ratio was down to 17. This increase in efficiency results in part from a reduction in draft animals, in part from a shift from ruminants to monogastrics, which rely little on pasture, and in part from an increased use of high quality feed from cropland for ruminants. It also results from improvements in animal husbandry, but we cannot break out the separate components (25).

Regional HANPP Trends.

HANPP has grown in all world regions at a slower rate than population, and all regions experienced a declining significance of land use-induced productivity losses (HANPPluc) and a growing share of harvested NPP in HANPP (Fig. 3). Otherwise, the specific patterns of HANPP differ substantially. Asia, Africa, and Latin America experienced very high growth rates in HANPP; as a percentage, HANPP doubled or even tripled in these regions during the last century. With the expansion of agriculture, these regions caught up with or even surpassed the initially high HANPP percentage levels in the Western Industrialized region and the former Soviet Union and Eastern Europe (FSU-EE). In contrast, in the Western Industrialized region, HANPP grew only modestly. It rose from 18% to 23% of NPPpot in the 1980s and has stabilized since then. The development of HANPP in FSU-EE mostly tracked that in the Western Industrial region until 1990, but after the collapse of the Communist system and the disintegration of its agricultural production system, HANPP rapidly declined from 22% to 16% of NPPpot.
Fig. 3.
Development of HANPP and HANPP per capita from 1910 to 2005 in five world regions. HANPP (percent) measures HANPP as a percentage of the NPP of the potential vegetation, i.e., the vegetation assumed to exist in the absence of land use. Asia*, Asia excluding those countries which are part of the FSU-EE Region; FSU-EE, Former Soviet Union and Eastern Europe. See SI Appendix for definition of regions.
HANPP as a percentage of NPPpot has converged globally and falls into a relatively narrow range in all regions except Asia (ranging from 16% to 23% in 2005), but per capita HANPP varies greatly (Fig. 3). HANPP per capita reflects three key factors: one, the amount and mix of biomass products consumed per capita, which generally increases with income and consumption of more HANPP-intensive products such as meat and milk; two, the efficiency of biomass production relative to NPPpot; and three, net biomass imports or exports. Some of the factors that drive per capita HANPP are shown in SI Appendix, Table S1:
  • i) Latin America has the highest HANPP per capita (5.8 tC/cap per y) because it has a relatively high level of biomass consumption, has only moderate yields compared with Asia, Europe, and North America, is a major world exporter, and produces a great deal of beef through relatively unproductive pasture from former forests, which entails a large HANPPluc.
  • ii) Asia has the lowest HANPP per capita (1.3 tC/cap per y). This low figure results from an intensive and high-yielding production system, a low role for livestock products in diets, a lower-than-average level of wood consumption, and a heavy reliance on imports.
  • iii) Africa is not only the region with the steepest increase in total HANPP, it also experienced a fast decline in HANPP per capita from 5.8 to 2.6 tC/cap per y. This decline is not comforting. The growth in HANPPluc is one measure of inefficiency of land use, and HANPPluc has been growing at faster rates in Africa than in any other region. HANPPharv has also increased, but the growth rate has still been much smaller than that of Africa’s rapidly growing population for a number of reasons: the number of livestock per capita declined considerably, yields have remained low, and the region has increased its reliance on imports of food.
  • iv) In the Western Industrial region, a very high level of biomass consumption, high exports, and a considerable density of livestock are counterbalanced by a highly efficient production system and a resulting large decline of HANPPluc over time. HANPP per capita amounted to 3.5 tC/cap per y in 2005. It declined only moderately in the 20th century and remained more or less stable after 1980. Together with Asia, the Western Industrial region has the most HANPP-efficient biomass production system. The ratio of total HANPP to harvest in this region is 30% below the global average because of the lowest HANPPluc.

Future Scenarios.

The historic trends in the relationship of HANPP to population, GDP, and bioenergy use allow us to project five potential future scenarios for the development of HANPP until 2050 based on these trends (Fig. 4; SI Appendix):
  • i) Scenario A projects HANPP based on the Organisation for Economic Co-operation and Development estimation that global economic output will grow by 246% between 2005 and 2050 (7). It also assumes a decline of 66% in the ratio of HANPP per dollar of global GDP based on the historic trend.
  • ii) Scenario B extrapolates HANPP on the basis of population forecasts for each of the five world regions by using the medium variant of United Nations projection of 43% population growth between 2005 and 2050 (6). It projects a decline of HANPP per capita based on the regional trend lines.
  • iii) Scenario C extrapolates HANPP from the assumptions that future demand for biomass products will follow population growth rates, that final biomass consumption per capita will remain constant at 0.3 tC/cap per y, and that HANPP per unit of final biomass consumption will decline by 26% toward the level observed in the Asia region, which has the lowest level of all five world regions.
  • iv) Scenarios D and E are based on the intermediate scenario B but assume additional primary bioenergy production. Based on potential deployment levels of biomass for energy identified by the Intergovernmental Panel on Climate Change-Special Report on Renewable Energy Sources and Climate Change Mitigation (IPCC-SRREN) (10), we calculated a lower and an upper boundary value for biomass harvest for energy production in 2050: Scenario D assumes an additional 50 EJ/y and Scenario E an additional 250 EJ/y of primary bioenergy over the present level of approximately 50 EJ/y (26). We further assumed that agricultural biomass will supply 60% and forest biomass 40% of the increase, and that HANPP per unit of agricultural biomass harvest further declines by 32% based on historical trends. This trend implies a continued growth in production efficiency, which could include circumstances in which energy crop plantations achieve an NPP that exceeds native productivity (NPPpot).
Fig. 4.
Scenarios for the development on HANPP until 2050. Whereas scenarios A–C assume a continuation of past trends, scenarios D and E add additional primary biomass harvest to scenario B (see text and SI Appendix for details). Based on upper and lower boundary values for deployment levels of biomass for energy, we assumed an additional harvest for energy production of 50 EJ/y (scenario D) and 250 EJ/y (scenario E) over the present value. Continuation of past trends would result in moderate growth of HANPP until 2050. Increasing the production of bioenergy, however, could dramatically increase global HANPP (scenario E).
In effect, all scenarios assume continued progress in HANPP efficiency by using different metrics, and two scenarios add a growth in bioenergy. In the first three scenarios, we project that HANPP will rise modestly from 25% to between 27% and 29%. These impacts are small in percentage terms, but because the human impact on the biosphere is already so great, the increases of 7–17% of human appropriation of the world’s productive capacity still implies meaningful human impacts on land resources. The big change would be the high bioenergy scenario, which implies a growth in HANPP to 44%; that is, a 78% increase over the present value. That increase would occur despite growth in efficiencies of biomass production to 2050 based on historic progress.
The significance of these impacts must be based on the degree of stress caused by present biomass demand. According to the Food and Agriculture Organization (FAO), irrigated areas have expanded from 1.5 to 3.1 million km2 in the last 50 y (27) and water withdrawal for agricultural use has increased fivefold during the last century (28). Humans have doubled the reactive nitrogen in the environment (29) and invested large amounts of fossil energy in agricultural production (SI Appendix, Fig. S3). Agricultural area has reached 5–6 billion hectares depending on the definition of pasture area. Any further large expansion of agricultural area would likely have vast significance for the global carbon cycle and biodiversity (4, 9).

Discussion

Although growing human needs for food and feed could roughly be met during the last century by expanding cultivated land and increasing yields, our results, at the most basic level, show rising human pressures on the terrestrial biosphere despite large increases in land use efficiency. This rising pressure is a cause for future concern, given mounting evidence that humanity is already undermining the ability of global ecosystems to maintain vital ecosystem services (30) and has arguably trespassed critical planetary boundaries for biodiversity loss and release of reactive nitrogen (12).
At the same time, this rise in HANPP has been far smaller than would have occurred if agricultural yields had not risen and if per capita bioenergy demands had not declined. Cropland yield gains, measured in HANPPharv on cropland as a ratio of NPPpot, increased from 41% to 69%. That increase, spread out over all cropland in 2005, generated 2.5 GtC/y of crops, which met 49% of the total increase in human consumption from 1910. Although the importance of rising yields has been well known, HANPP provides a useful measure of these efficiency gains because it equates all crops based on their carbon content, relates it to the productivity in global land ecosystems and, hence, demonstrates the magnitude of human-induced changes to the global carbon cycle.
Our calculations also provide appropriate recognition of the importance of harvested crop residues. Their consumption has increased from 0.5 petagram of carbon (PgC)/y to 1.6 PgC/y even as crops have increased from 0.3 PgC/y to 1.8 PgC/y. This benefit grows in parallel with the growth in crop yields, and their importance cautions against the treatment of crop residues as if they were unused.
Although there are concerns about the increasing reliance of agriculture on energy use, our calculations indicate that, in pure energy terms, gains in output were larger than increases in inputs. Researchers have debated the relative contribution of fertilizer, plant breeding, irrigation, and other land improvements toward yield gains, but they generally conclude that the changes are more interactive than additive. For example, increased fertilizer has facilitated yield gains that require other measures as well but would not have been possible without fertilizer (31). Overall, we calculate that total energy used in agriculture both directly and for the production of fertilizer reached 13 EJ by 2005 (SI Appendix, Fig. S3), but the energy in crops and crop residues rose from 41 EJ in 1910 to 155 EJ in 2005. However, ecological costs of agricultural intensification go far beyond increased energy inputs and include impacts such as soil degradation, nutrient leaching, greenhouse gas emissions, and biodiversity loss (32, 33).
Our analysis also suggests the importance of focusing in the future on pasture productivity. Unlike crops, there is no evidence to support comparable increases in pasture productivity on larger scales. Indeed, the expansion of pasture on original forest land and soil degradation on grassland have resulted in an increase in HANPPluc, although the exact magnitude of this NPP loss is difficult to gauge with currently available data (SI Appendix). Further improvements in land use efficiency may depend heavily on improvements in pasture management, which are a focus of some climate change strategies (34).

Conclusions

For the next few decades, a further increase in global population and economic output is expected, and they will raise the demand for more biomass to produce food, fiber, and fuel. Our analysis of historic trends has shown that considerable efficiency gains in the past have driven a decoupling of socio-economic growth and HANPP, but only relative to population and GDP growth. In absolute terms, HANPP has continued to increase. Overall, people have to a fair extent managed to improve the efficiency with which they generate their food and fiber needs, but even with these improvements, the total tap on the world’s plant production has roughly doubled and the ecological costs were considerable. Even if these trends continue, HANPP is likely to increase significantly without increased reliance on bioenergy. Bioenergy at levels contemplated by the International Energy Agency (35) and in IPCC-SRREN (10) would have a transformative effect on the planet. As the world faces large new demands for food and timber products, that experience suggests caution in refocusing the energy economy on bioenergy, and stresses the importance of developing improved practices for sustainable intensification of land use (9, 33).

Materials and Methods

We refer to the concept of HANPP used in our previous work (17) and adapted the methodology used therein for application to historical time periods. Defining HANPP as the sum of HANPPharv and HANPPluc, we calculate HANPP for nine points in time (1910, 1930, 1950, 1960, 1970, 1980, 1990, 2000, and 2005) for up to 161 individual countries aggregated to five regions. At the global scale for the period 1961–2005, we also calculated a time series in annual resolution.
We use model runs of LPJ for managed lands, a biogeochemical process model of climate-dependent carbon and water dynamics in vegetation growth, to estimate NPPpot. HANPPharv includes biomass extracted for further economic use and biomass killed by harvest and by human-induced fires. The method to calculate biomass harvest is adapted from previous work (3, 36). Data on used extraction of crops and timber come from FAO and its precursor (SI Appendix). For the years 1910 and 1930, primary data are not available for all countries. We extrapolate total flows for each region from information on reporting countries and their relative contribution to the total regional flow in 1950. Grazed biomass was estimated on the basis of feed balances by using livestock and market feed data from FAO and demand factors that considered species, region, and time. Grazed biomass is calculated as the difference between modeled dry matter demand and available market feed, fodder crops, and by products used as feed. Extraction of crop residues, harvest losses in forestry, and below-ground biomass on cropland and harvested forest areas are estimated by using region and time-dependent coefficients. The amount of biomass killed in human-induced fires (deforestation) was taken from the literature (37), complemented by an estimate of biomass killed in swidden agriculture (SI Appendix).
HANPPluc is the difference between NPPpot and NPPact, i.e., the productivity of the vegetation prevailing at each point in time. Negative values of HANPPluc indicate that fertilization or irrigation raised productivity above its natural level. NPPact on cropland is extrapolated from crop harvest and calculated crop residues. We use coefficients to estimate belowground NPP and NPP losses during the growing season (SI Appendix). We assume that HANPPluc on artificial grassland (grassland on areas with potential forest cover) was 20% of NPPpot (17); estimates of HANPPluc due to human-induced degradation come from data from a previous study for the year 2000 (38), extrapolated backward by assuming that the ratio between HANPPluc and grazed NPPharv is not changing. This approach yields similar results as the combination of spatially explicit datasets on degradation extent and degree for the late 20th century (38, 39) with time series of NPPpotand pasture land (40), which we take as an indication that our basic approach is valid, given the large data gaps.
HANPPluc on natural grasslands, on forest, and on unused land (e.g., wilderness areas) is assumed to be zero. The extent of land used for infrastructure, buildings, and associated areas like gardens or parks relies on population data and per capita values and an assumption that the amount of built-up land varies with income and population density by region and over time (SI Appendix). HANPPharv on built-up land (e.g., mowing lawns and cutting trees) is assumed to be 50% of NPPact (as in ref. 17).

Acknowledgments

This work was supported by Austrian Science Funds Projects P20812-G11 and P21012-G11, European Union–Seventh Framework Programme Project 265104 (Visions of Land Use Transitions in Europe), the Social Sciences and Humanities Research Council of Canada, and European Research Council Starting Grant An integrated socio-ecological approach to land-use intensity: Analysing and mapping biophysical stocks/flows and their socioeconomic drivers (LUISE) 263522. This work contributes to the Global Land Project (www.globallandproject.org).

Footnotes

  • Author contributions: F.K., K.-H.E., and H.H. designed research; F.K., K.-H.E., S.G., H.H., A.B., V.G., C.L., and C.P. performed research; F.K., K.-H.E., S.G., H.H., V.G., C.L., C.P., and T.D.S. analyzed data; and F.K., K.-H.E., H.H., and T.D.S. wrote the paper.
  • The authors declare no conflict of interest.
  • This article is a PNAS Direct Submission. W.L. is a guest editor invited by the Editorial Board.
  • This article contains supporting information online at www.pnas.org/lookup/suppl/doi:10.1073/pnas.1211349110/-/DCSupplemental.
Freely available online through the PNAS open access option.

References

  1. ↵
  2. ↵
  3. ↵
  4. ↵
  5. ↵
  6. ↵
  7. ↵
  8. ↵
  9. ↵
  10. ↵
  11. ↵
  12. ↵
  13. ↵
  14. ↵
  15. ↵
  16. ↵
  17. ↵
  18. ↵
  19. ↵
  20. ↵
  21. ↵
  22. ↵
  23. ↵
  24. ↵
  25. ↵
  26. ↵
  27. ↵
  28. ↵
  29. ↵
  30. ↵
  31. ↵
  32. ↵
  33. ↵
  34. ↵
  35. ↵
  36. ↵
  37. ↵
  38. ↵
  39. ↵
  40. ↵